Abstract
Microsatellite (SSR) markers were employed to investigate the genetic diversity within a collection of durum wheat germplasm. A total of 41 landraces originating from geographically diverse regions—including Turkey, Lebanon, Morocco, Ethiopia, China, Kazakhstan, and Mongolia—were initially genotyped using 27 SSR markers selected to represent the whole genome. Of these, 7 markers failed to produce amplification products despite repeated attempts; therefore, 20 SSR markers were retained for further analysis. Among these, 17 loci were polymorphic and 3 were monomorphic.
Analysis of the 17 polymorphic loci revealed a total of 67 alleles, with allele numbers per locus ranging from two to seven and an average of 3.94 alleles per locus. The polymorphic information content (PIC) values varied from 0.071 (Xgwm371) to 0.647 (Xgwm120), indicating differences in marker informativeness.
Cluster analysis grouped the landraces into four genetically distinct clusters, demonstrating a clear relationship between genetic variation and geographic origin. In general, landraces from Africa and Western Asia exhibited higher genetic diversity compared to those from Central and East Asia. These results highlight Western Asia, Africa, and particularly southeastern Turkey as important centers of genetic diversity for durum wheat.
-
Key words: Durum Wheat, Genetic Diversity, SSR Markers, Polymorphism
Introduction
Durum wheat (
Triticum turgidum ssp.
durum) ranks as the tenth most widely cultivated cereal crop globally, with an estimated annual production of approximately 38 million tons (
Xynias et al. 2020). The Mediterranean region dominates global output, contributing nearly 75% of the total. However, its cultivation extends well beyond this area, with substantial production reported in countries such as Canada, Mexico, the United States, Russia, Kazakhstan, Azerbaijan, and India (
De Vita et al. 2019;
Martínez-Moreno et al. 2022). Within the Triticum genus, durum wheat is considered the second most significant species after bread wheat (
Triticum aestivum), accounting for around 10-11% of the global wheat cultivation area and contributing roughly 5-6% to total wheat production (
Bekhshfard et al. 2009;
Beres et al. 2020;
Mohammadi et al. 2022).
One major factor limiting the wider adoption of durum wheat compared to bread wheat is its narrower genetic base. As a tetraploid species, durum wheat lacks the D-genome present in hexaploid bread wheat, which restricts its genetic diversity. While landraces display extensive and regionally structured variability—particularly in the Mediterranean and Middle Eastern regions—modern cultivars tend to possess a much-reduced gene pool. Additionally, many durum varieties are cold-sensitive and have a spring growth habit, which restricts their adaptability to diverse agro-climatic conditions. Furthermore, durum wheat typically yields about 20% less than bread wheat (
Johnson et al. 2021;
Mammadova et al. 2024b).
Local landraces represent a vital reservoir of genetic diversity, shaped by centuries of natural and human selection (
Alizada et al. 2020;
Bagheri et al. 2026;
Mammadova et al. 2021). These traditional varieties hold valuable alleles that contribute to plant resilience, including tolerance to drought, heat, and various diseases (
Alizade et al. 2025;
Ganeva et al. 2010;
Mammadova et al. 2026). Given climate change projections—which suggest that the Mediterranean could lose up to 19% of its suitable durum wheat growing area by mid-century and as much as 48% by 2100—there is an urgent need to explore and utilize this genetic wealth (
Dagnaw et al. 2023). Genomic tools and participatory breeding approaches can help unlock this potential.
Accordingly, the present study aims to assess and compare the genetic diversity of durum wheat landraces collected from different geographical regions, with the goal of identifying genotypes possessing valuable traits for future breeding efforts.
Materials and Methods
In this study, a total of 41 durum wheat landraces from seven geographic regions worldwide, all obtained from ICARDA, were examined (
Table 1).
Genomic DNA was extracted from young leaf tissues of each durum wheat cultivar using the cetyltrimethylammonium bromide (CTAB) method as described by
Doyle et al. (1987). To assess genetic diversity, a total of 17 simple sequence repeat (SSR) markers were utilized. The markers were selected to ensure genome-wide coverage, with at least one primer pair positioned on each chromosome.
Polymerase chain reaction (PCR) amplifications were performed in a total reaction volume of 15 μL. Each reaction mixture contained 2 μL of genomic DNA (at a concentration of 50 ng/μL), 1.5 μL of 10× PCR buffer, 1 μL of a 0.67 mM dNTP mix, 1 unit of Taq DNA polymerase, and 1 μL each of forward and reverse primers (2 μM concentration).
PCR conditions followed the protocol outlined by
Röder et al. (1998), consisting of 45 cycles with the following parameters: initial denaturation at 94℃ for 1 minute, annealing at 55℃ or 60℃ (depending on the primer pair) for 1 minute, and extension at 72℃ for 1 minute. A final extension was carried out at 72℃ for 5 minutes.
The amplification products were resolved on a 6% denaturing polyacrylamide gel via electrophoresis. Band visualization was achieved using silver staining. SSR alleles were scored in a binary format, with the presence and absence of bands recorded as ‘1’ and ‘0’, respectively.
Genetic similarity among genotypes was calculated based on Jaccard’s similarity coefficient (
Jaccard 1908). The resulting similarity matrix was used to construct a dendrogram using the Unweighted Pair Group Method with Arithmetic Mean (UPGMA), implemented through the statistical software packages PAST and PowerMarker. PAST software was used to perform the clustering and generate dendrograms for classifying all genotypes based on genetic similarity, while PowerMarker was used for clustering among populations.
The genetic parameters—Polymorphism Information Content (PIC), Probability of Identity (PI), and Discrimination Power (D)—were calculated to evaluate the effectiveness and informativeness of the SSR markers used in the study. These parameters were computed using the following formulas:
PIC=1 - Σpi2
PI=Σpi4 + ΣΣ(2PiPj)2
D=1 - PI
Where Pi and Pj are the frequencies of the ith and jth SSR alleles, respectively.
To evaluate the relationship between agronomic traits and molecular marker data, independent sample t-tests were conducted. All statistical analyses were performed using SPSS software, version 19.0.
The agronomic traits were measured in a field experiment conducted at the Genetic Resources Institute of Azerbaijan. A total of 41 durum wheat landraces were evaluated using a randomized complete block design (RCBD) with three replications. Standard agronomic practices were applied, and the traits—including days to maturity and 1000-grain weight—were recorded following conventional measurement procedures.
Results
After two attempts, no amplification products were obtained for seven SSR markers—Xbarc83, Cfd59, Cfa220, Xcfa2086, Xgwm108, Xgwm124, and Wmc364—among the 27 SSRs analyzed. Accordingly, 20 SSRs were assayed further in the 41 germplasms (
Table 2).
Among the 20 SSR markers analyzed, 17 loci were polymorphic, while 3 (Xgwm1045, Xgwm750, and Xgwm126) were monomorphic. Across the 17 polymorphic markers, a total of 67 alleles were detected, with an average of 3.94 alleles per locus. The highest allele numbers were observed at the Xgwm146 (7 alleles), Xgwm540 (6 alleles), and Xgwm526 (6 alleles) loci. In contrast, the Xgwm251 and Xgwm371 loci each exhibited only two alleles among the samples. The highest polymorphism information content (PIC) values were recorded for Xgwm120 (0.647), Xgwm526 (0.616), and Xgwm540 (0.607), indicating their greater informativeness among the evaluated genotypes.
These markers with minimum values of PI and maximum values of D have also been able to identify genotypes more effectively (
Table 3).
Correlation analysis revealed associations between the assessed agronomic traits and specific microsatellite alleles (
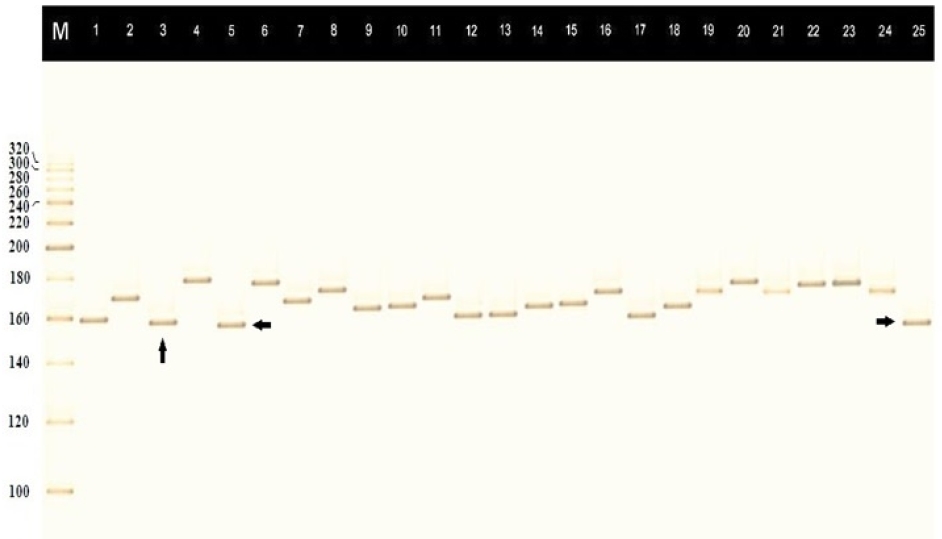
Table 4). At the Xgwm540 locus, the 159-bp allele was detected exclusively in genotypes China 1, 3, and 5; Ethiopia 1 and 4; and Kazakhstan 1 and 5 (
Fig. 1). These genotypes exhibited a lower average number of days to maturity (183.38 days) compared to the remaining 34 genotypes carrying alternative alleles at this locus (200.58 days). This suggests that the 159-bp allele of Xgwm540 may serve as a potential marker for early-maturing genotypes.
Although early-maturing varieties typically have lower yields than late-maturing ones, early ripening is particularly important in regions where avoiding end-of-season drought, diseases, or pest pressure is critical, or where a second crop is grown after wheat harvest. In addition, a significant association was observed between the Xgwm120 locus and the 1000-grain weight trait (
Table 4).
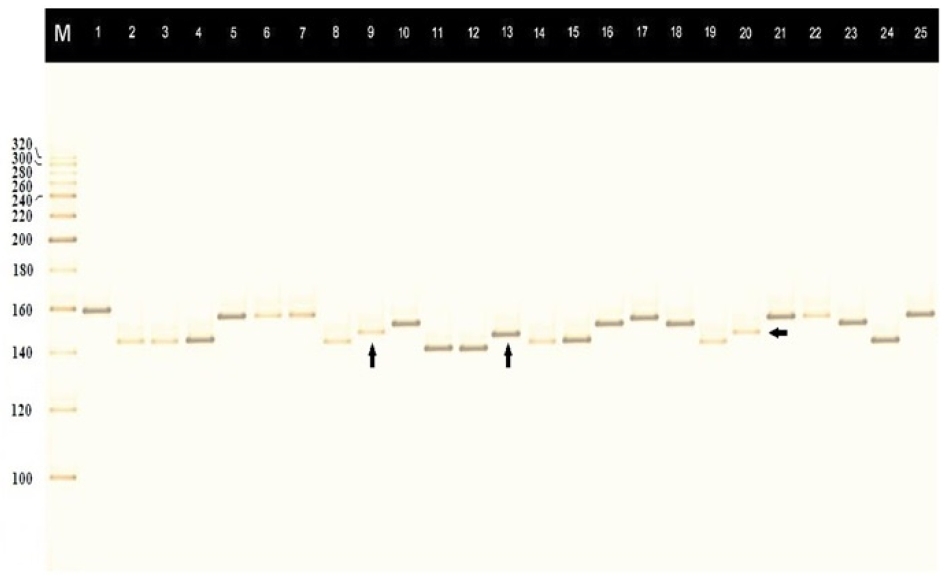
Genotypes Turkey 3, Lebanon 1, Morocco 2, Ethiopia 2, and Kazakhstan 4, all carrying the 149-bp allele at the Xgwm120 locus (
Fig. 2), showed a higher average 1000-grain weight (50.19 g) compared to the remaining 36 genotypes with other alleles at this locus, which had an average grain weight of 37.96 g. However, further validation is required before these two loci can be proposed as reliable genetic markers.
Genetic analysis based on microsatellite markers indicated that, in the South-East Turkish durum wheat population, an average of more than 2.76 alleles per marker was observed. The overall genetic diversity index for this population was 0.529.
The results compared with those of other study populations suggested that the wheat samples of South-East Turkey were the most diverse population. According to the markers used, the probability of identity in this population was 0.341. This indicates that not all SSR markers were equally informative for discriminating genotypes within the South-East Turkish population, as some loci exhibited low polymorphism or identical banding patterns. Among the markers examined, Xgwm120, with five alleles, a PIC value of 0.777, and a PI value of 0.083, was the most informative primer for assessing genetic diversity among the samples. In contrast, Xgwm264 and Xgwm371, each producing a single monomorphic band, did not reveal any polymorphism within the population.
For Xgwm674, two alleles were detected. In addition, single unique alleles were observed for Xgwm169 (188-bp), Xgwm120 (145-bp), Xgwm526 (208-bp, 202-bp), and Xgwm146 (220-bp), and these were found exclusively in the South-East Turkish samples. For the Xgwm156 marker, a total of three alleles were identified, with all allelic variants present in the Turkish samples. In comparison, other populations exhibited only one or at most two alleles for this marker.
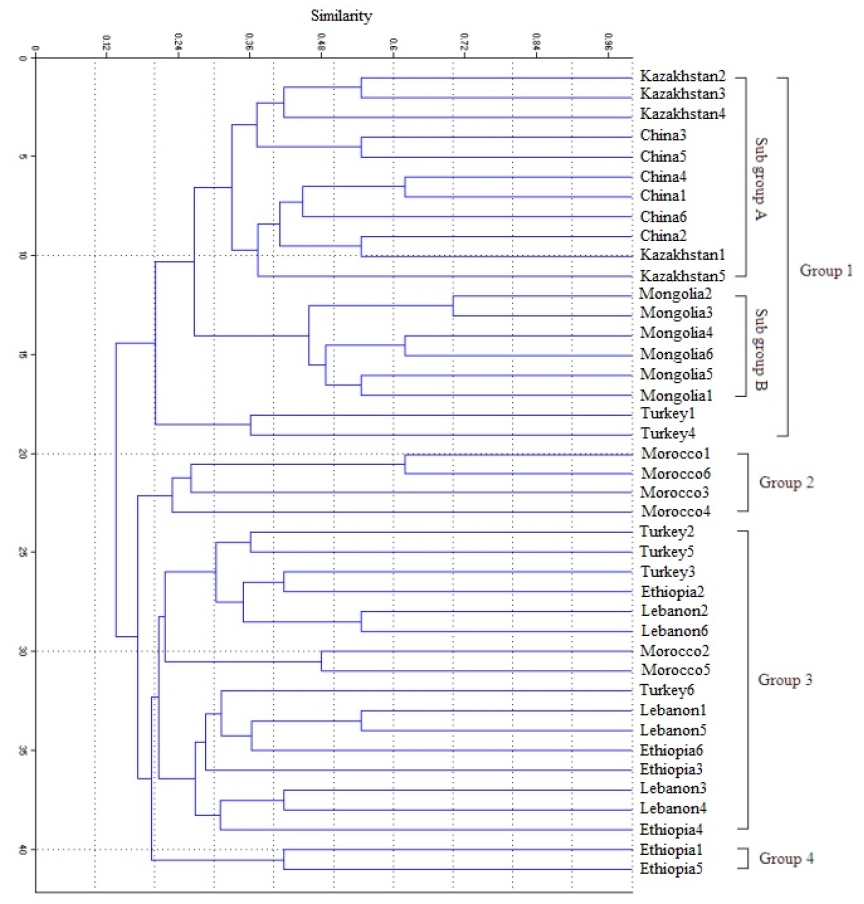
Cluster analysis showed that genotypes 1 and 4 from South-East Turkey were separated from other West Asian wheat samples and clustered together with samples from China, Mongolia, and Kazakhstan in Group I (
Fig. 3). In contrast, genotypes 2, 3, 5, and 6 from the same population were grouped in Group III.
Among the studied populations, Ethiopian and Lebanese samples showed the closest genetic relationships to South-East Turkish genotypes, with genetic distance coefficients of 0.110 and 0.119, respectively. In contrast, wheat populations from China, Mongolia, and Kazakhstan were the most genetically distant from the Turkish samples (
Table 5).
The Xgwm120 locus was the most informative marker for assessing diversity in Lebanese durum wheat, revealing four alleles with a PI value of 0.128 and a PIC value of 0.722. Although Lebanese samples showed a relatively low average number of alleles (2.29) and a genetic diversity index of 0.444, they were less diverse than South-East Turkish and African populations but more diverse than Central and East Asian populations (China, Mongolia, and Kazakhstan;
Table 3). All Lebanese genotypes were assigned to Group III (
Fig. 3).
The genetic distance analysis indicated that Ethiopian and Turkish populations showed the closest genetic relationships to the Lebanese genotypes, with coefficients of 0.114 and 0.119, respectively. In contrast, the Kazakh population exhibited the greatest genetic distance from the Lebanese samples (coefficient = 0.305). For the Moroccan durum wheat population, similar to Lebanon, the Xgwm120 locus was identified as the most informative marker. Moroccan samples showed an average of 2.35 alleles per locus; although this was lower than that observed in South-East Turkish durum wheat, their genetic diversity indices were comparable (
Table 3). Cluster analysis revealed that Moroccan genotypes 1, 3, 4, and 6 grouped in Cluster II, while the remaining two genotypes clustered in Group III. Overall, Moroccan wheat samples showed the highest similarity with Ethiopian, Turkish, and Lebanese populations, while being most genetically distant from Kazakh and Mongolian populations (
Table 5).
For Ethiopian durum wheat samples, the average number of alleles and genetic diversity index were 2.35 and 0.49, respectively. The Xgwm526 and Xgwm120 markers were identified as the most informative loci for assessing genetic variation in this population. In contrast, Xgwm371 and Xgwm251 were monomorphic and did not reveal any polymorphism among Ethiopian samples.
More than 66% of Ethiopian genotypes were grouped in Cluster III (
Fig. 3), whereas genotypes 1 and 5 were assigned to Cluster IV, indicating their genetic distinctiveness from the remaining Ethiopian samples and from other studied populations.
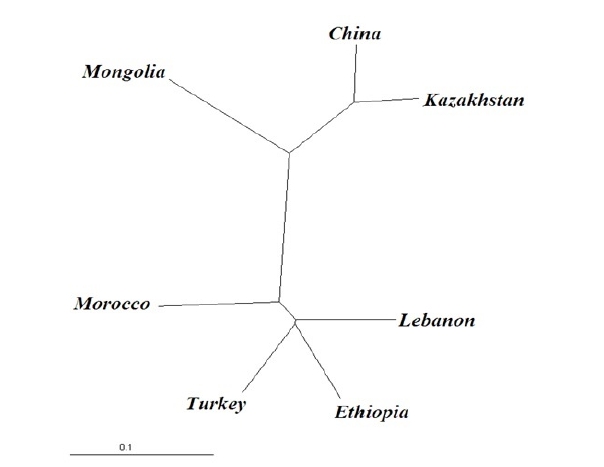
Across all genotypes, Ethiopian genotype No. 5 and Kazakh genotype No. 3 showed the greatest genetic distance, with a similarity coefficient of 0.14. Overall, Ethiopian samples were genetically closest to South-East Turkish, Lebanese, and Moroccan populations, while showing the greatest divergence from Kazakh, Chinese, and Mongolian populations (
Fig. 4).
The genetic diversity index and average number of alleles in Chinese durum wheat samples were 0.366 and 1.88, respectively, while for Kazakhstan they were 0.367 and 1.94. These results indicate that both Chinese and Kazakh populations exhibit lower genetic diversity compared to Western Asian (Turkey and Lebanon) and African (Morocco and Ethiopia) populations. All Chinese and Kazakh genotypes were grouped in Sub-group A of Cluster I, reflecting their high genetic similarity. This pattern was further supported by genetic distance analysis, which showed that Kazakhstan and China were the closest populations, with a genetic distance of 0.074.
For Chinese durum wheat, the most informative SSR markers were Xgwm526, Xgwm540, and Xgwm132, while for the Kazakh population, Xgwm120, Xgwm540, and Xgwm146 were the most suitable loci for diversity assessment.
Mongolian durum wheat exhibited the lowest genetic diversity among all studied populations, with an average number of alleles of 1.7 and a genetic diversity index of 0.248. Although Xgwm526 and Xgwm540 showed moderate polymorphism in this population (three alleles, PIC = 0.499, PI = 0.302), seven SSR markers were monomorphic. All Mongolian genotypes were assigned to Sub-group B of Cluster I. In addition, genotypes 2 and 3 from Mongolia were the most similar within the population, with a similarity coefficient of 0.7. Overall, genetic distance analysis indicated that Chinese genotypes were closest to Lebanese and Ethiopian populations, whereas Mongolian durum wheat was the most genetically distant among all studied populations.
Discussion
Overall, the results indicate that in many cases, genotypes originating from the same geographic region tended to cluster together, and populations from geographically closer regions showed higher genetic similarity. This suggests that genetic diversity in the studied germplasm is, to a considerable extent, structured according to geographic origin.
The results further showed that populations from Western Asia (South-East Turkey and Lebanon) and Africa (Morocco and Ethiopia) exhibited relatively higher genetic diversity compared to populations from Central and East Asia (China, Mongolia, and Kazakhstan). Among all studied groups, the South-East Turkish durum wheat population showed comparatively high genetic diversity and also possessed alleles at five loci that were not detected in other populations. These findings suggest that this population may harbor unique genetic variation and highlights its potential importance for durum wheat germplasm conservation and breeding. Similar observations regarding the genetic diversity of durum wheat and its wild progenitor (
T. dicoccoides) in Southeast Turkey have been reported in previous studies (
Luo et al. 2007;
Mori et al. 2003;
Ozkan et al. 2002;
Ozkan et al. 2005;
Salamini et al. 2002;
Zohary et al. 2000).
Phylogenetic evidence from previous studies indicates the existence of two main races of
T. dicoccoides: a Western race distributed in Israel, Syria, Lebanon, and Jordan, and a Central-Eastern race found mainly in Turkey and less frequently in Iraq and Iran. The Central-Eastern race is considered to have contributed significantly to the domesticated durum wheat gene pool. This hypothesis is supported by studies on Karacadag populations in Turkey, which show phylogenetic patterns consistent with progenitor-domesticated relationships (
Luo et al. 2007;
Mori et al. 2003;
Ozkan et al. 2002). From this region, emmer wheat likely spread into Asia, Europe, and Africa (
Dubrovsky et al. 2007;
Kong et al. 2004).
Overall, the germplasm from different countries represents an important genetic resource containing alleles for agronomically important traits such as stress tolerance and yield potential. The relatively lower genetic diversity observed in Chinese and Kazakh populations compared to Western Asian and African populations was confirmed by both allele number and genetic diversity indices. In contrast, Mongolian durum wheat showed the lowest genetic diversity among all studied populations. Genetic distance analysis further indicated that Chinese and Kazakh populations were closely related, while Mongolian genotypes were the most genetically distant.
In summary, populations from South-East Turkey, Lebanon, Morocco, and Ethiopia generally exhibited higher genetic diversity compared to those from Central and East Asia. The presence of unique alleles in the South-East Turkish population suggests the presence of distinct genetic variation that may be valuable for future germplasm utilization, although further validation in broader datasets is required.
Fig. 1.Amplification pattern of alleles from Xgwm540 separated through polyacrylamide gel electrophoresis. M: 20 bp Ladder, 1-6: Durum wheat from China, 7-12: Durum wheat from South-East Turkey, 13-18: Durum wheat from Lebanon, 19-24: Durum wheat from Morocco, 25: Durum wheat from Ethiopia. SSR marker (159-bp) is indicated with an arrow (only the relevant part of the representative gel is shown).
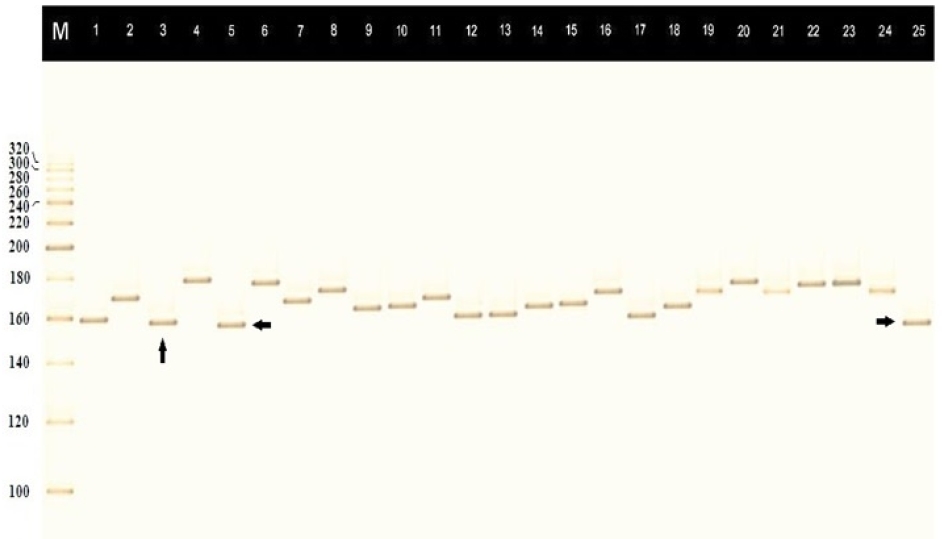
Fig. 2.Amplification pattern of alleles from Xgwm120 separated through polyacrylamide gel electrophoresis. M: 20 bp Ladder, 1-6: Durum wheat from China, 7-12: Durum wheat from South-East Turkey, 13-18: Durum wheat from Lebanon, 19-24: Durum wheat from Morocco, 25: Durum wheat from Ethiopia. SSR marker (149-bp) is indicated with an arrow (only the relevant part of the representative gel is shown).
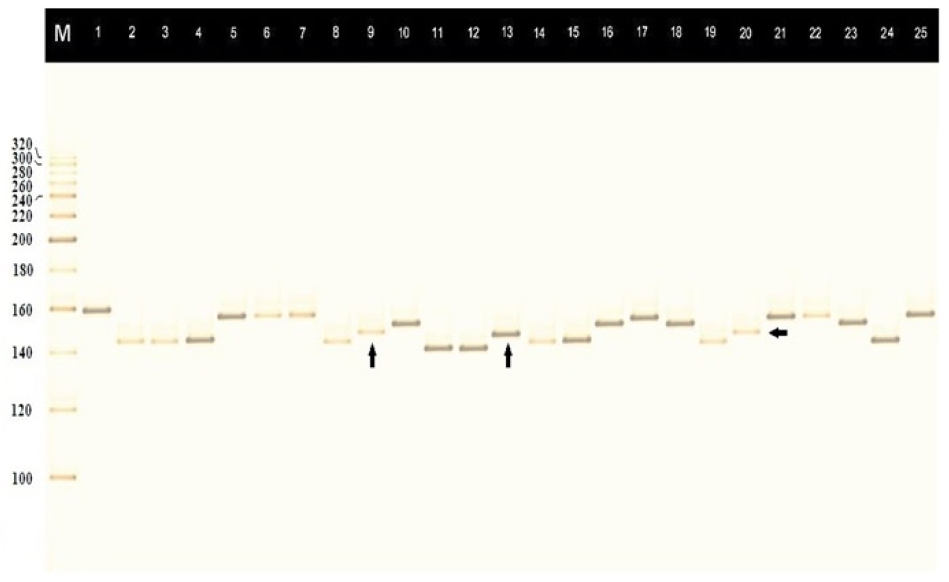
Fig. 3.Dendrogram showing the relationship among 41 genotypes of durum wheat based on SSR markers.
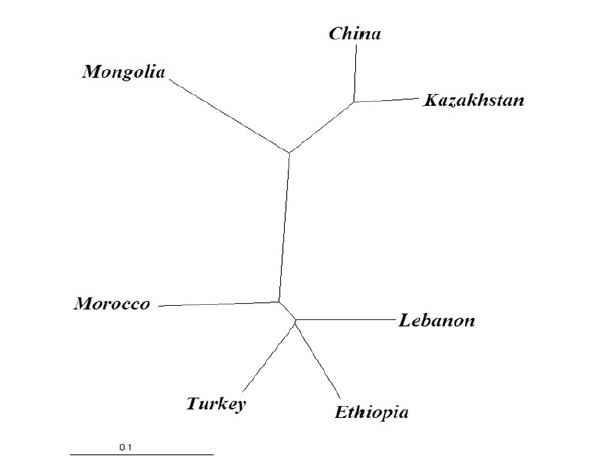
Fig. 4.Dendrogram showing the genetic distance among studied durum wheat populations based on SSR markers.
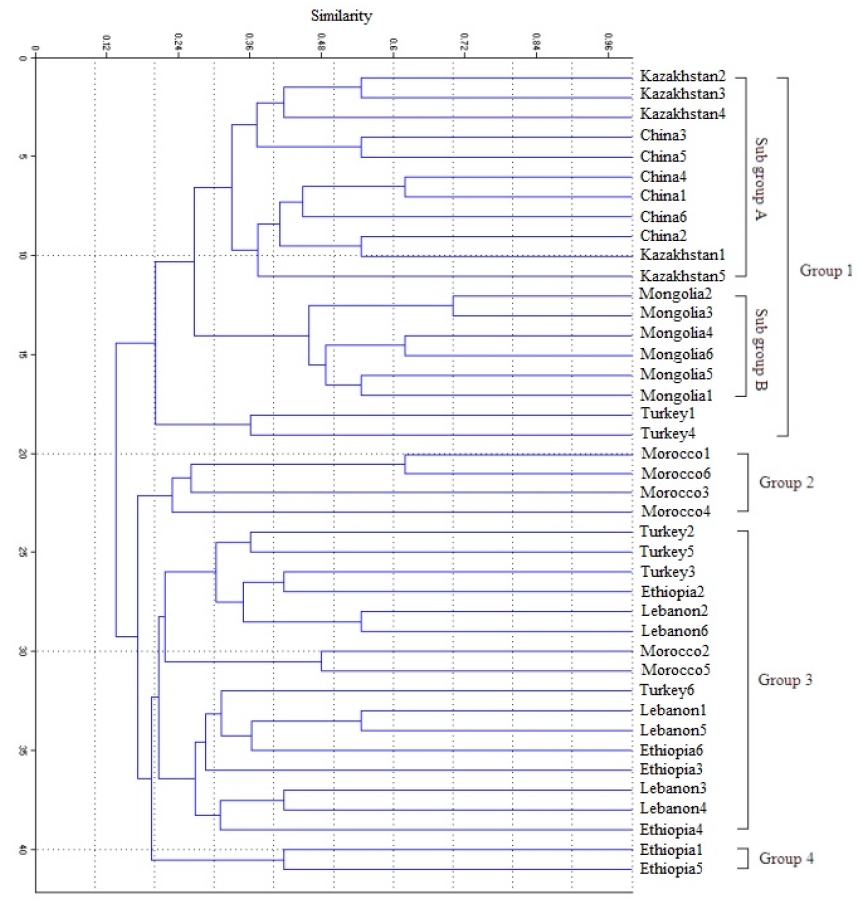
Table 1.Details on the genotypes used for assessing molecular diversity.
Table 1.
|
Genotypes |
Collecting region |
Longitude |
Latitude |
Genotypes |
Collecting region |
Longitude |
Latitude |
|
Turkey3 |
Van |
37°45' N |
43°02' E |
Lebanon2 |
Ynouh |
33°15' N |
35°18' E |
|
Ethiopia4 |
Bale |
7°15' N |
39°32' E |
Morocco6 |
Boulemane |
33°07' N |
4°29' W |
|
China1 |
Tibet |
29°46' N |
84°01' E |
Kazakhstan2 |
Balkhash District |
45°42' N |
74°20' E |
|
China2 |
Tibet |
29°58' N |
84°30' E |
China6 |
Tibet |
29°21' N |
87°32' E |
|
Morocco2 |
Jerada |
33°48' N |
2°10' W |
Ethiopia2 |
Jimma |
8°04' N |
37°16' E |
|
Turkey4 |
Shirnak |
37°45' N |
42°53' E |
Kazakhstan3 |
Moiynkum District |
45°02' N |
73°55' E |
|
Ethiopia6 |
Bale |
6°53' N |
38°59' E |
Lebanon1 |
Touline |
33°14' N |
35°26' E |
|
Kazakhstan5 |
Shet District |
46°50' N |
73°23' E |
Morocco5 |
Sefrou |
33°38' N |
4°30' W |
|
Lebanon3 |
Nabatieh |
33°28' N |
35°26' E |
Mongolia6 |
Burd |
47°08' N |
104°04' E |
|
China3 |
Tibet |
31°04' N |
85°12' E |
Turkey1 |
Van |
37°49' N |
42°52' E |
|
Ethiopia1 |
East Shewa |
9°04' N |
39°43' E |
Mongolia2 |
Khuld |
45°15' N |
105°30' E |
|
Ethiopia5 |
Shinile |
9°31' N |
41°16' E |
Turkey6 |
Siirt |
37°46' N |
41°44' E |
|
Lebanon4 |
Roumine |
33°28' N |
35°26' E |
Mongolia3 |
Manlai |
44°22' N |
107°17' E |
|
Morocco3 |
Taourirt |
33°58' N |
2°58' W |
Kazakhstan4 |
Moiynkum District |
44°35' N |
72°00' E |
|
Lebanon5 |
Kfar Melki |
33°29' N |
35°29' E |
Morocco4 |
Khenifra |
32°49' N |
4°54' W |
|
China4 |
Tibet |
30°44' N |
86°30' E |
Mongolia4 |
Zagiin us |
44°35' N |
106°38' E |
|
Morocco1 |
Taza |
33°59' N |
4°07' W |
Mongolia5 |
Dornogovi |
46°16' N |
108°51' E |
|
Kazakhstan1 |
Shet District |
46°31' N |
71°59' E |
China5 |
Tibet |
28°42' N |
85°18' E |
|
Lebanon6 |
Rihane |
33°26' N |
35°33' E |
Turkey2 |
Batman |
37°43' N |
41°14' E |
|
Mongolia1 |
Buren |
46°34' N |
105°13'E |
Turkey5 |
Diyarbakır |
37°46' N |
40°55' E |
|
Ethiopia3 |
East Gojjam |
10°18' N |
38°22' E |
|
|
|
|
Table 2.Characteristics of SSR markers used for the analysis of durum wheat populations.
Table 2.
|
SSR marker |
Repeats |
Chromosome location |
Annealing temperatures, ℃ |
|
Xgwm164 |
(CT)16 |
1A |
55 |
|
Xgwm249 |
(GA)11(GGA)8 |
2A |
55 |
|
Xgwm674 |
(CT)16CCC(GT)4 |
3A |
60 |
|
Xgwm165 |
(GA)20 |
4A |
60 |
|
Xgwm156 |
(GT)14 |
5A |
60 |
|
Xgwm169 |
(GA)23 |
6A |
60 |
|
Xgwm130 |
(GT)22 |
7A |
60 |
|
Xgwm264 |
(CA)9A(CA)24 |
1B |
60 |
|
Xgwm120 |
(CT)11(CA)18 |
2B |
60 |
|
Xgwm526 |
(CT)16 |
2B |
55 |
|
Xgwm340 |
(GA)26 |
3B |
60 |
|
Xgwm389 |
(CT)14(GT)16 |
3B |
60 |
|
Xgwm251 |
(CA)28 |
4B |
55 |
|
Xgwm371 |
(CA)10(GA)32 |
5B |
60 |
|
Xgwm540 |
(CT)3(CC)(CT)16 |
5B |
55 |
|
Xgwm132 |
(GA)24(GAA)6 |
6B |
60 |
|
Xgwm146 |
(GA)5GG(GA)20 |
7B |
60 |
Table 3.Genetic diversity of seven durum wheat populations detected by seventeen SSR markers.
Table 3.
|
Population |
Allele No. |
PIC |
PI |
D |
|
Turkey |
2.76 |
0.529 |
0.341 |
0.659 |
|
Lebanon |
2.29 |
0.444 |
0.431 |
0.569 |
|
Morocco |
2.35 |
0.529 |
0.330 |
0.670 |
|
Ethiopia |
2.35 |
0.490 |
0.385 |
0.615 |
|
China |
1.88 |
0.366 |
0.536 |
0.464 |
|
Mongolia |
1.70 |
0.284 |
0.629 |
0.371 |
|
Kazakhstan |
1.94 |
0.367 |
0.534 |
0.466 |
|
SSR marker |
|
|
|
|
|
Xgwm164 |
4 |
0.497 |
0.373 |
0.627 |
|
Xgwm249 |
3 |
0.465 |
0.417 |
0.583 |
|
Xgwm674 |
5 |
0.576 |
0.276 |
0.724 |
|
Xgwm165 |
2 |
0.269 |
0.652 |
0.348 |
|
Xgwm156 |
3 |
0.418 |
0.464 |
0.536 |
|
Xgwm169 |
5 |
0.521 |
0.337 |
0.663 |
|
Xgwm130 |
3 |
0.254 |
0.661 |
0.339 |
|
Xgwm264 |
3 |
0.198 |
0.741 |
0.259 |
|
Xgwm120 |
5 |
0.647 |
0.208 |
0.792 |
|
Xgwm526 |
6 |
0.616 |
0.226 |
0.774 |
|
Xgwm340 |
3 |
0.473 |
0.390 |
0.610 |
|
Xgwm389 |
3 |
0.481 |
0.385 |
0.615 |
|
Xgwm251 |
2 |
0.135 |
0.826 |
0.174 |
|
Xgwm371 |
2 |
0.071 |
0.911 |
0.089 |
|
Xgwm540 |
6 |
0.607 |
0.235 |
0.765 |
|
Xgwm132 |
5 |
0.521 |
0.339 |
0.661 |
|
Xgwm146 |
7 |
0.559 |
0.297 |
0.703 |
|
Mean |
3.94 |
0.430 |
0.455 |
0.545 |
Table 4.Genetic relationship between agronomical traits and SSR markers.
Table 4.
|
Traits |
SSR markers |
No. genotypes |
Mean |
SD |
F |
T-test |
|
Days to maturity |
Xgwm540 |
7 |
183.38 |
1.00 |
5.57 |
0.023 * |
|
34 |
200.58 |
7.42 |
|
1000-grain weight |
Xgwm120 |
5 |
50.19 |
0.67 |
5.17 |
0.029 * |
|
36 |
37.96 |
4.86 |
Table 5.Genetic distances among studied durum wheat populations based on SSR data.
Table 5.
|
Turkey |
Lebanon |
Morocco |
Ethiopia |
China |
Mongolia |
Kazakhstan |
|
Turkey |
0.000 |
|
|
|
|
|
|
|
Lebanon |
0.119 |
0.000 |
|
|
|
|
|
|
Morocco |
0.151 |
0.146 |
0.000 |
|
|
|
|
|
Ethiopia |
0.110 |
0.114 |
0.135 |
0.000 |
|
|
|
|
China |
0.266 |
0.270 |
0.193 |
0.262 |
0.000 |
|
|
|
Mongolia |
0.242 |
0.269 |
0.201 |
0.295 |
0.156 |
0.000 |
|
|
Kazakhstan |
0.250 |
0.305 |
0.204 |
0.286 |
0.074 |
0.189 |
0.000 |
References
- Achtar S, Mouaalla MY, Kalhout A, Röder MS, Mirali N. 2010. Assessment of genetic diversity among Syrian durum (Triticum turgidum ssp. durum) and bread wheat (Triticum aestivum L.) using SSR markers. Genetika. 46: 1500-1506.
- Akparov ZI, Mamedova RB, Guseynova LA, Abdulalieva GS, Yunusova FM, Alizade SA. 2021. Competitive evaluation of perspective cotton lines in variety development nursery. Adv. Curr. Nat. Sci. 10: 7-12.
- Alamerew S, Chebotar S, Huang X, Rӧder MS, Bӧrner A. 2004. Genetic diversity in Ethiopian hexaploid and tetraploid wheat germplasm assessed by microsatellite markers. Genet. Resour. Crop Evol. 51: 559-567.
- Alizada S, Guliev R, Mammadova R, Zaefizadeh M. 2020. System perspective analysis for molecular and genetic source of salt tolerance in cotton. Khazar J. Sci. Technol. 4(1): 70-83.
- Alizada Sh, Aliyeva K. 2024. Comparative analysis of expression profiles of antiporter encoding gene (GhNHX1) under different concentrations of NaCl in cotton (Gossypium hirsutum L.). Adv. Biology Earth Sci. 9(1): 168-174.
- Alizada S, Aliyeva K, Mammadova R, Bayramli O, Moghanloo B.S. 2024. Salinity, verticillium wilt tolerance and genetic diversity analysis of upland cotton genotypes. Adv. Biology Earth Sci. 9(2): 242-252.
- Alizade S, Mammadova R, Shirinova A, Amrahov N, Aghazada G, Javadzade A, et al. 2025. Evaluation of the effect of exogenous application of indole-3-acetic acid on morphophysiological parameters under salt (NaCl) stress in cotton(G. hirsutum L.). Adv. Biology Earth Sci. 10(1): 40-50.
- Bagheri F, Fakhari R, Mammadova R. 2026. Effect of accelerated aging of borage (Borago officinalis L.) seeds on seed reproduction and biochemical content. Yuz. Yil Univ. J. Agric. Sci. 2026(1): 1-13.
- Bekhshfard O, Naghavi MR, Mardi M, Bihamta MR, Kazemi M, Pirseyedi SM. 2009. A study of genetic diversity in durum wheat (Triticum turgidum) using microsatellite markers. Iran. J. Field Crop Sci. 40: 75-83.
- Ben Amer IM, Börner A, Röder MS. 2001. Detection of genetic diversity in Libyan wheat genotypes using wheat microsatellite markers. Genet. Resour. Crop Evol. 48: 579-585.
- Beres BL, Rahmani E, Clarke JM, Grassini P, Pozniak CJ, Geddes CM, et al. 2020. A systematic review of durum wheat: Enhancing production systems by exploring genotype, environment, and management (G× E× M) synergies. Front. Plant Sci. 11: 568657.
- Dagnaw T, Mulugeta B, Haileselassie T, Geleta M, Ortiz R, Kassahun T. 2023. Genetic diversity of durum wheat (Triticum turgidum L. ssp. durum, Desf) germplasm as revealed by morphological and SSR markers. Genes. 14(6): 1155.
- De Vita P, Taranto F. 2019. Durum wheat (Triticum turgidum ssp. durum) breeding to meet the challenge of climate change. In Advances in plant breeding strategies: cereals (Vol, 5, pp. 471-524). Cham: Springer International Publishing.
- Doyle JJ, Doyle JL. 1987. A rapid DNA isolation procedure for small quantities of fresh leaf tissue. Phytochem. Bull. 19: 11-15.
- Dubrovsky J, Dvorak J. 2007. Genome plasticity a key factor in the success of polyploid wheat under domestication. Science. 316: 1862-1866.
- Ganeva G, Korzun V, Landjeva S, Popova Z, Christov NK. 2010. Genetic diversity assessment of Bulgarian durum wheat(Triticum durum Desf.) landraces and modern cultivars using microsatellite markers. Genet. Resour. Crop Evol. 57: 273-285.
- Huang XQ, Bӧrner A, Rӧder MS, Ganal MW. 2002. Assessing genetic diversity of wheat (Triticum aestivum L.) germplasm using microsatellite markers. Theor. Appl. Genet. 105: 699-707.
- Jaccard P. 1908. Nouvelles recherches sur la distribution florale. Bull. Soc. Vaudoise Sci. Nat. 44: 223-270.
- Johnson R, Green T, White P. 2021. Advances in breeding cold-tolerant durum wheat. Agric. Res. J. 20(2): 78-95. https://doi.org/10.5678/arj.2021.0023
- Kong XY, Gu YQ, You FM, Dubrovsky J, Anderson OD. 2004. Dynamics of the evolution of orthologous and paralogous portions of a complex locus region in two genomes of all-polyploid wheat. Plant Mol. Biol. 54: 55-69.
- Luo MC, Yang ZL, You FM, Kawahara T, Waines JG, Dvorak J. 2007. The structure of wild and domesticated emmer wheat populations, gene flow between them, and the site of emmer domestication. Theor. Appl. Genet. 114: 947-959.
- Maccaferri M, Sanguineti MC, Donini P, Tuberosa R. 2003. Microsatellite analysis reveals a progressive widening of the genetic basis in the elite durum wheat germplasm. Theor. Appl. Genet. 107: 783-797.
- Mammadova R, Akparov Z, Amri A, Bakhsh A, Alo F, Alizade S, et al. 2024b. Genetic diversity analysis of Azerbaijani bread wheat (Triticum aestivum L.) genotypes with simple sequence repeat markers linked to drought tolerance. Genet. Resour. Crop Evol. 72(1): 315-323.
- Mammadova R, Amri A, Akparov Z, Alo F, Sheikhzamanova F, Abbasov M, et al. 2024a. Evaluation of genetic diversity using SSR markers and link with drought response of Azerbaijani durum wheat (Triticum durum Desf.) genotypes. Genet. Resour. Crop Evol. 71(5): 2203-2212.
- Mammadova R, Huseynova L, Abdulaliyeva G, Yunusova F, Alizade S. 2021. Prospects of the remote hybridization on improvement of the main economical traits of cotton genotypes with naturally colored fibre. East Eur. Sci. J. 1(6): 4-8.
- Mammadova R, Salimov V, Alizade S, Amrahov N. 2025. Evaluation of genetic diversity of azerbaijani grape varieties (Vitis ssp.) by using ISSR markers. Plant Breed. Biotechnol. 13: 167-175.
- Mammadova R, Salimov V, Trapp O, Alizade SH, Röckel F. 2026. Genetic analysis of grapevine (Vitis vinifera L.) genotypes from Azerbaijan using simple sequence repeat markers. Genet. Resour. Crop Evol. 73: 23.
- Martínez-Moreno F, Giraldo P, Cátedra MDM, Ruiz M. 2021. Evaluation of leaf rust resistance in the Spanish core collection of tetraploid wheat landraces and association with ecogeographical variables. Agriculture. 11: 277.
- Mohammadi R, Haghparast R. 2022. Durum wheat: Production, nutritional value and economic importance. Cereal Biotechnol. Biochem. 1(3): 414-445.
- Mori N, Ishii T, Ishido T, Hirosawa S, Watatani H, Kawahara T, et al. 2003. Origin of domesticated emmer and common wheat inferred from chloroplast DNA fingerprinting. In Proc. 10th. Int. Wheat Genetics Symp., Paestum. 25-28
- Ojaghi J, Nurieva S, Salayeva S, Eldarov M, Akparov Z, Eldarova J. 2025. Allelic diversity of Azerbaijan bread wheat (Triticum aestivum L.) by SSR markers. Turk. J. Agric. For. 49(2): 397-404.
- Salamini F. 2005. A reconsideration of the domestication geography of tetraploid wheats. Theor. Appl. Genet. 110: 1052-1060.
- Ozkan H, Brandolini A, Schaffer-Pregl R, Salamini F. 2002. AFLP analysis of a collection of tetraploid wheats indicates the origin of emmer and hard wheat domestication in southeast Turkey. Mol. Biol. Evol. 19(10): 1797-1801.
- Rӧder MS, Korzun V, Wendehake K, Plaschke J, Tixer MH, Leory P, et al. 1998. A microsatellite map of wheat. Genetics. 149: 2007-2023.
- Salamini F, Özkan H, Brandolini A, Schäfer-Pregl R, Martin W. 2002. Genetics and geography of wild cereal domestication in the near east. Nat. Rev. Genet. 3(6): 429-441.
- Salimov V, Huseynova A, Guliyeva A, Alizade A, Mammadova R. 2025. Assessment of biomorphological and economically important traits of some local grape varieties and clones of Azerbaijan. Adv. Biology Earth Sci. 10(2): 303-313.
- Salimov V, Mammadova R, Burak M, Alizade S, Sharifova S, Bakhsh A, et al. 2024. Inter simple sequence repeat (ISSR) based genetic and morphological polymorphism of Azerbaijani grape (Vitis vinifera) genotypes. Genet. Resour. Crop Evol. 2711-2723.
- Xynias IN, Mylonas I, Korpetis EG, Ninou E, Tsaballa A, Avdikos ID, et al. 2020. Durum wheat breeding in the Mediterranean region: Current status and future prospects. Agronomy. 10(3): 432.
- Yang X, Tan B, Liu H, Zhu W, Xu L, Wang Y, et al. 2020. Genetic diversity and population structure of Asian and European common wheat accessions based on genotyping-by-sequencing. Front. Genet. 11: 580782.
- Yifru TY, Hammer K, Huang XQ, Rӧder MS. 2006. Regional patterns of microsatellite diversity in Ethiopian tetraploid wheat accessions. Plant Breed. 125(2): 125-130.
- Zohary D, Hopf M. 2000. Domestication of plants in the Old World. 3rd edn. 316pp. New York: Oxford University Press. £ 19.95 (softback). Ann. Bot. 88(4): 666.